LEVPTDGNAGLLAEPQIAMFCGKLNMHMNVQNGKWESDPSGTKTCIGTKEGILQYCQEVYPELQITNVVEANQPVTIQNWCKRGRKQCKTHTHIVIPYRCLVGEFVSDALLVPDKCKFLHQERMDVCETHLHWHTVAKETCSEKSTNLHDYGMLLPCGIDKFRGVEFVCCPLAEESDSIDSADAEEDDSDVWWGGADTDYADGGEDKVVEVAEEEEVADVEEEEAEDDEDVEDGDEVEEEAEEPYEEATERTTSIATTTTTTTESVEEVVREVCSEQAETGPCRAMISRWYFDVTEGKCAPFFYGGCGGNRNNFDTEEYCMAVCGSVSSQSLLKTTSEPLPQDPVKLPTTAASTPDAVDKYLETPGDENEHAHFQKAKERLEAKHRERMSQVMREWEEAERQAKNLPKADKKAVIQHFQEKVESLEQEAANERQQLVETHMARVEAMLNDRRRLALENYITALQAVPPRPHHVFNMLKKYVRAEQKDRQHTLKHFEHVRMVDPKKAAQIRSQVMTHLRVIYERMNQSLSLLYNVPAVAEEIQDEVDELLQKEQNYSDDVLANMISEPRISYGNDALMPSLTETKTTVELLPVNGEFSLDDLQPWHPFGVDSVPANTENEVEPVDARPAADRGLTTRPGSGLTNIKTEEISEVKMDAEFGHDSGFEVRHQKLVFFAEDVGSNKGAIIGLMVGGVVIATVIVITLVMLKKKQYTSIHHGVVEVDAAVTPEERHLSKMQQNGYENPTYKFFEQMQN
Note: The complete
sequence may include tag sequence, target protein sequence, linker sequence and extra sequence that is
translated with the protein sequence for the purpose(s) of secretion, stability, solubility, etc.
If the exact amino acid sequence of this recombinant protein is critical to your application,
please explicitly request the full and complete sequence of this protein before ordering.
Protein Length
Full Length of Mature Protein
Tag Info
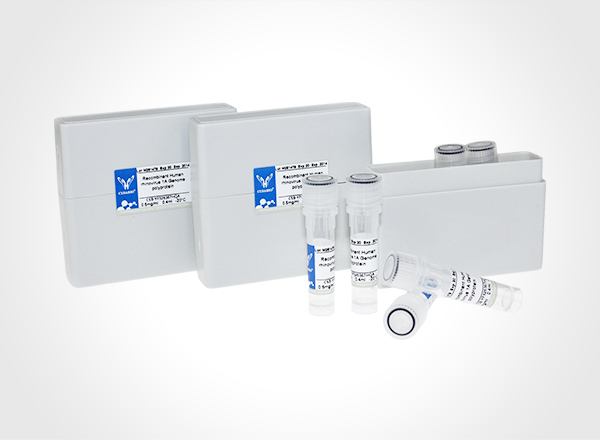
N-terminal 10xHis-tagged
The tag type will be determined during production process. If you have specified tag type, please tell us and we will develop the specified tag preferentially.
Storage Condition
Store at -20°C, for extended storage, conserve at -20°C or -80°C.
Shelf Life
The shelf life is related to many factors, storage state, buffer ingredients, storage temperature and the stability of the protein itself.
Generally, the shelf life of liquid form is 6 months at -20°C/-80°C. The shelf life of lyophilized form is 12 months at -20°C/-80°C.
Notes
Repeated freezing and thawing is not recommended. Store working aliquots at 4°C for up to one week.
Functions as a cell surface receptor and performs physiological functions on the surface of neurons relevant to neurite growth, neuronal adhesion and axonogenesis. Interaction between APP molecules on neighboring cells promotes synaptogenesis. Involved in cell mobility and transcription regulation through protein-protein interactions. Can promote transcription activation through binding to APBB1-KAT5 and inhibit Notch signaling through interaction with Numb. Couples to apoptosis-inducing pathways such as those mediated by G(O) and JIP. Inhibits G(o) alpha ATPase activity. Acts as a kinesin I membrane receptor, mediating the axonal transport of beta-secretase and presenilin 1. By acting as a kinesin I membrane receptor, plays a role in axonal anterograde transport of cargo towards synapes in axons. May be involved in copper homeostasis/oxidative stress through copper ion reduction. Can regulate neurite outgrowth through binding to components of the extracellular matrix such as heparin and collagen I and IV. The splice isoforms that contain the BPTI domain possess protease inhibitor activity. Induces a AGER-dependent pathway that involves activation of p38 MAPK, resulting in internalization of amyloid-beta peptide and leading to mitochondrial dysfunction in cultured mitochondrial dysfunction in cultured cortical neurons. Provides Cu(2+) ions for GPC1 which are required for release of nitric oxide (NO) and subsequent degradation of the heparan sulfate chains on GPC1.; Amyloid-beta peptides are lipophilic metal chelators with metal-reducing activity. Binds transient metals such as copper, zinc and iron. Rat and mouse amyloid-beta peptides bind only weakly transient metals and have little reducing activity due to substitutions of transient metal chelating residues. Amyloid-beta protein 42 may activate mononuclear phagocytes in the brain and elicits inflammatory responses. Promotes both tau aggregation and TPK II-mediated phosphorylation. Also binds GPC1 in lipid rafts.; Appicans elicit adhesion of neural cells to the extracellular matrix and may regulate neurite outgrowth in the brain.; The gamma-CTF peptides as well as the caspase-cleaved peptides, including C31, are potent enhancers of neuronal apoptosis.; N-APP binds TNFRSF21 triggering caspase activation and degeneration of both neuronal cell bodies (via caspase-3) and axons (via caspase-6).
Gene References into Functions
These results, in Wistar rats, provide experimental support for the hypothesis that certain risk factors, such as energy metabolism dysfunction or the aging process itself, may increase vulnerability to beta-amyloid protein (Abeta). Hippocampal region is more susceptible to Abeta and its effect increases with age in relation to the neocortex.PMID:29624358
Abeta 25-35 was found to induce PC12 cell apoptosis in a dose-dependent manner (P<0.05). Moreover, Abeta 25-35 also caused dose-dependent disintegration of the cytoskeleton (P<0.05).PMID:29436599
Andrographolide (ANDRO) reduced inflammation-mediated neuronal damage by blocking inflammatory responses of microglial cells to Abeta(1-42), suggesting ANDRO may be an effective agent in modulating neuroinflammatory process in Alzheimer's disease.PMID:28669260
alanine in APP- intracellular domain(ICD) and the proline in APLP2-ICD lie directly behind a conserved caspase cleavage sitePMID:26921470
These data suggest that methylation change in BDNF exon is involved in the regulation of BDNF expression by Abeta or SAM, and further support the view of specific epigenetic modifications of a certain BDNF gene transcript.PMID:29305263
Results from the present study indicated that pioglitazone may improve insulin sensitivity and ameliorate Abeta42 accumulation in rats with dietinduced IR by regulating AKT/GSK3beta activation, suggesting that pioglitazone may be a promising drug for AD treatment.PMID:28447730
Dynamic transport of Abeta aggregates is only observed between axon terminal and cell body. In addition to differential cellular uptake, more Abeta-peptide secretion is detected significantly from axons than from dendritic side.PMID:28121396
Results show that concerted signaling by both APP and Abeta is necessary for aberrant neuronal cell cycle entry. Thus, APP plays a central role in promotion of neurodegeneration, through activation of Ras-ERK signaling axis as well as GSK-3, and interfering with these signaling events would impede cell cycle reentry and neurodegeneration observed in Alzheimer's disease.PMID:28374012
Lynx1 and Abeta1-42 bind competitively to multiple nicotinic acetylcholine receptor subtypes.PMID:27460145
increased APP and/or beta-CTF impact the endocytic pathway to disrupt NGF trafficking and signaling, resulting in trophic deficits in basal forebrain cholinergic neurons.PMID:27064279
results establish a novel toxic impact ofAbeta oligomers on neuronal metabolism and suggest that Abeta oligomers-induced, NMDA receptor-mediated AMPK inhibition may play a key role in early brain metabolic defects in AD.PMID:28302722
The protein level of Abeta in serum and cerebrospinal fluid (CSF) was severity and timedependent during the acute phase in rats with traumatic spinal cord injury (SCI). Monitoring the level of Abeta protein in serum may improve the evaluation of SCI severity and the neuron functional status following SCI.PMID:28259979
O3 exposure (0.25 ppm) induced a significant increase of Syntaxin 5 and accumulation of betaA42 peptide in the reticulum in cells of the dentate gyrusPMID:27366738
results indicate that specifically "trapping" low-n oligomers provides a novel strategy for toxic Abeta42-oligomer recognition and removal.PMID:26510576
Results indicate that improving synaptic soluble AbetaPPalpha availability at synapses helps in reducing the functional NMDAR-related deregulation of hippocampal networks linked to agingPMID:26402095
High glucose leads to the increased expression of genes related to Abeta production, resulting in the accumulation of Abeta in the lens.PMID:27028062
Autoimmune Optic Neuritis Is Associated with Altered APP Cleavage in Neurons and Up-Regulation of p53PMID:26426258
Redox-mediated posttranslational modification of brain proteins link Abeta and hyperglycaemia to cognitive dysfunction in metabolic syndrome/type 2 diabetes and Alzheimer disease.PMID:26743041
This study indicates that interfering intracellular Abeta especially mitochondrial Abeta accumulation, together with ameliorating Abeta-associated mitochondrial dysfunction, may contribute to the protective effects of huperzine A against Abeta neurotoxicity.PMID:26024517
Syt-1 and Syt-9 regulate endogenous APP-CTF and Abeta levels in PC12 cells. Secreted sAPPbeta levels were significantly reduced in PC12 cells lacking Syt-1 expression.PMID:26202512
Results show that downregulation of let-7d might contribute to isoflurane-induced learning and memory impairment through upregulating its target APP, and increasing the production of Abeta subsequently.PMID:25799420
Exposure to As-, Cd-, and Pb-mixture induces Abeta, amyloidogenic APP processing and cognitive impairments via oxidative stress-dependent neuroinflammation in young rats.PMID:25288670
Data suggests that APP is important in regulating intestinal cholesterol uptake in a fashion dependent upon specific proteolytic pathways.PMID:25742317
The soluble extracellular fragment of neuroligin-1 protects synapses in neurons damaged by ABETA oligomers.PMID:26325471
The present study indicates that Abeta-mediated Zn2+ influx into dentate granule cells, which may occur without AMPA receptor activation, transiently induces a short-term cognitive deficit.PMID:25536033
Incubation of brain homogenates with 70 microM hydrogen peroxide significantly influenced the profile of Abeta binding proteins and 0.1 mM isatin decreased the number of identified Abeta binding proteins.PMID:25551598
Abeta-40 Y10F exhibited remarkably decreased neurotoxicity compared to Abeta-40 which could be partly due to the reduced generation of hydrogen peroxide.PMID:22754299
The results of this study provide the first direct demonstration that AbetaPP is mostly distributed among glutamatergic rather than GABAergic or cholinergic terminals of the adult rat hippocampus.PMID:24531160
report we describe a novel neuroprotective function of mGlu3 receptors related to their ability to promote the non-amyloidogenic pathway of APP cleavage in astrocytes, thus enhancing sAPPalpha productionPMID:24291464
Rodent-Abeta staining is present and increased after juvenile traumatic brain injury around cerebral blood microvessels, and the diameter of those is decreased by 25% and 34% at 2 and 6 months, respectively, without significant angiogenesis.PMID:25052558
Oxidative stress served as the key trigger to down-regulate miR-107 by cell- derived soluble Abeta.PMID:24595404
present results suggest that the amyloid peptide exhibits a protective antioxidant role in biological systems, but also has toxic actions independent of oxidative stressPMID:23041348
Both voltage-activated Ca2+ channel and NMDAR-dependent long-term potentiation in vivo are strongly inhibited by Abeta.PMID:24298149
the existence of a structurally related family of quasi-fibrillar conformers of Abeta42, which is stabilized both by curcumin and by Zn(2+.)PMID:24599958
analysis of the role of JIP1 in APP transport; knockdown of JIP1 did not affect either amyloid precursor protein transport or amyloid-beta peptide productionPMID:23825109
Data suggest that the brain expression of neprilysin may promote amyloid beta-protein (Abeta)deposition in patients with Alzheimer's disease (AD).PMID:24508800
Neurodegeneration may occur in a retrograde fashion from axon terminals near beta-amyloid plaques which may spread through brain regions in cortical neuron cultures.PMID:24114864
APP is an independently operating cell adhesion moleculePMID:23691241
These data present novel insights into the subsynaptic localization of APPsPMID:23815291
Abeta42 globulomers have an antiparallel beta-sheet arrangementPMID:23687299
processing of amyloid precursor protein in cells undergoing apoptosisPMID:23469123
Identification of the minimal zinc-binding center in natural isoforms of amyloid-beta domain 1-16 using ESI-MSPMID:23888782
results showed that EMP exposure can cause long-term impairment in impaired cognition and memory of rats, resulting in AD-like symptoms; this may be induced by enhancing oxidative stress and is related to autophagy dysfunctionPMID:23523687
The CentA1-Ras-Elk-1 signaling pathway acts on mitochondria to regulate dendritic spine density and synaptic plasticity in response to Abeta in hippocampal neurons.PMID:23516302
Prion protein-mediated toxicity of amyloid-beta oligomers requires lipid rafts and the transmembrane LRP1PMID:23386614
Neuronal binding and hippocampal neurotransmission were found to be suitable to account for the synaptotoxicity to different App assemblies, based on the stability of the applied App aggregates in these settings.PMID:23374097
Early brain injury alters the blood-brain barrier phenotype in parallel with beta-amyloid and cognitive changes in adulthood.PMID:23149553
S-nitrosylation pathway wherein Cdk5/NOS1 interaction enhances S-nitrosylation of Cdk5, mediates mitochondrial dysfunction and synaptic loss during the App etiology of Alzheimer's disease.PMID:22874667
C1q-induced LRP1B and GPR6 proteins expressed early in Alzheimer disease mouse models, are essential for the C1q-mediated protection against amyloid-beta neurotoxicityPMID:23150673
Show
More
Hide
All
Subcellular Location
Cell membrane; Single-pass type I membrane protein. Membrane; Single-pass type I membrane protein. Perikaryon. Cell projection, growth cone. Membrane, clathrin-coated pit. Early endosome. Cytoplasmic vesicle.; [C83]: Endoplasmic reticulum. Golgi apparatus. Early endosome.; [C99]: Early endosome.; [Amyloid-beta protein 42]: Cell surface.; [Gamma-secretase C-terminal fragment 59]: Nucleus. Cytoplasm.; [Soluble APP-beta]: Secreted.
Protein Families
APP family
Tissue Specificity
Expressed in the brain. In the brain, non-L-APP isoforms are expressed in neurons, isoform APP695 being the predominant form. In astrocytes and microglial cells, almost 50% is L-isoform (appican).