LEVPTDGNAGLLAEPQIAMFCGKLNMHMNVQNGKWESDPSGTKTCIGTKEGILQYCQEVYPELQITNVVEANQPVTIQNWCKRGRKQCKTHTHIVIPYRCLVGEFVSDALLVPDKCKFLHQERMDVCETHLHWHTVAKETCSEKSTNLHDYGMLLPCGIDKFRGVEFVCCPLAEESDSVDSADAEEDDSDVWWGGADTDYADGGEDKVVEVAEEEEVADVEEEEADDDEDVEDGDEVEEEAEEPYEEATERTTSTATTTTTTTESVEEVVREVCSEQAETGPCRAMISRWYFDVTEGKCVPFFYGGCGGNRNNFDTEEYCMAVCGSVSTQSLLKTTSEPLPQDPDKLPTTAASTPDAVDKYLETPGDENEHAHFQKAKERLEAKHRERMSQVMREWEEAERQAKNLPKADKKAVIQHFQEKVESLEQEAANERQQLVETHMARVEAMLNDRRRLALENYITALQAVPPRPHHVFNMLKKYVRAEQKDRQHTLKHFEHVRMVDPKKAAQIRSQVMTHLRVIYERMNQSLSLLYNVPAVAEEIQDEVDELLQKEQNYSDDVLANMISEPRISYGNDALMPSLTETKTTVELLPVNGEFSLDDLQPWHPFGVDSVPANTENEVEPVDARPAADRGLTTRPGSGLTNIKTEEISEVKMDAEFGHDSGFEVRHQKLVFFAEDVGSNKGAIIGLMVGGVVIATVIVITLVMLKKKQYTSIHHGVVEVDAAVTPEERHLSKMQQNGYENPTYKFFEQMQN
Note: The complete
sequence may include tag sequence, target protein sequence, linker sequence and extra sequence that is
translated with the protein sequence for the purpose(s) of secretion, stability, solubility, etc.
If the exact amino acid sequence of this recombinant protein is critical to your application,
please explicitly request the full and complete sequence of this protein before ordering.
Protein Length
Full Length of Mature Protein
Tag Info
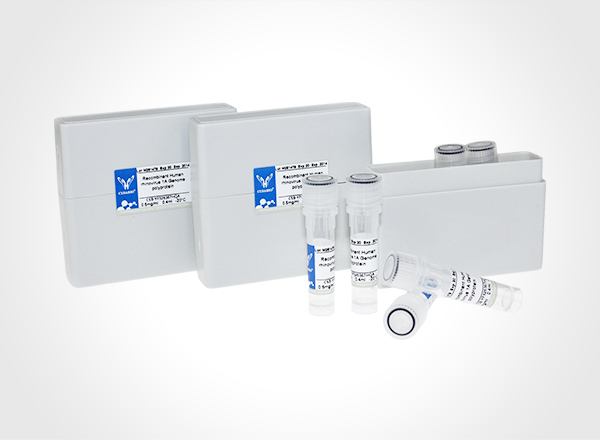
N-terminal 10xHis-tagged
The tag type will be determined during production process. If you have specified tag type, please tell us and we will develop the specified tag preferentially.
Buffer
Lyophilized from Tris/PBS-based buffer, 6% Trehalose, pH 8
Storage Condition
The shelf life is related to many factors, storage state, buffer ingredients, storage temperature and the stability of the protein itself. Generally, the shelf life of liquid form is 6 months at -20°C/-80°C. The shelf life of lyophilized form is 12 months at -20°C/-80°C.
Shelf Life
The shelf life is related to many factors, storage state, buffer ingredients, storage temperature and the stability of the protein itself.
Generally, the shelf life of liquid form is 6 months at -20°C/-80°C. The shelf life of lyophilized form is 12 months at -20°C/-80°C.
Notes
Repeated freezing and thawing is not recommended. Store working aliquots at 4°C for up to one week.
Functions as a cell surface receptor and performs physiological functions on the surface of neurons relevant to neurite growth, neuronal adhesion and axonogenesis. Interaction between APP molecules on neighboring cells promotes synaptogenesis. Involved in cell mobility and transcription regulation through protein-protein interactions. Can promote transcription activation through binding to APBB1-KAT5 and inhibit Notch signaling through interaction with Numb. Couples to apoptosis-inducing pathways such as those mediated by G(O) and JIP. Inhibits G(o) alpha ATPase activity. Acts as a kinesin I membrane receptor, mediating the axonal transport of beta-secretase and presenilin 1. By acting as a kinesin I membrane receptor, plays a role in axonal anterograde transport of cargo towards synapes in axons. May be involved in copper homeostasis/oxidative stress through copper ion reduction. Can regulate neurite outgrowth through binding to components of the extracellular matrix such as heparin and collagen I and IV. The splice isoforms that contain the BPTI domain possess protease inhibitor activity. Induces a AGER-dependent pathway that involves activation of p38 MAPK, resulting in internalization of amyloid-beta peptide and leading to mitochondrial dysfunction in cultured cortical neurons. Provides Cu(2+) ions for GPC1 which are required for release of nitric oxide (NO) and subsequent degradation of the heparan sulfate chains on GPC1.; Amyloid-beta peptides are lipophilic metal chelators with metal-reducing activity. Binds transient metals such as copper, zinc and iron. Rat and mouse amyloid-beta peptides bind only weakly transient metals and have little reducing activity due to substitutions of transient metal chelating residues. Amyloid-beta protein 42 may activate mononuclear phagocytes in the brain and elicit inflammatory responses. Promotes both tau aggregation and TPK II-mediated phosphorylation. Also binds GPC1 in lipid rafts.; The gamma-CTF peptides as well as the caspase-cleaved peptides, including C31, are potent enhancers of neuronal apoptosis.; N-APP binds TNFRSF21 triggering caspase activation and degeneration of both neuronal cell bodies (via caspase-3) and axons (via caspase-6).
Gene References into Functions
This study uncovered two clear phases in the life of APP23 mice: developmental and aging. Development displays similarities to young carriers of familial Alzheimer's disease (AD) mutations. All gene expression differences between APP23 and control mice correlate with aging. Age-related expression changes appear exacerbated/accelerated in APP23 mice.PMID:27838490
These results provide evidence for an emerging role of BAG-1M in the regulation of BACE1 expression and AD pathogenesis and that targeting the BAG-1M-NF-kappaB complex may provide a mechanism for inhibiting Abeta production and plaque formation.PMID:28502705
Conformational changes in a mouse model of Alzheimer's disease-linked amyloid beta and APP take place before the amyloids plaques can be seen.PMID:28287086
These results support the proposition that Aβ release during thrombosis serves as part of a natural defense against infection.PMID:29890636
These data suggest a novel regulatory function of juxta- and intra-membrane domains on the metabolism and function of APP.PMID:29777707
Inflammasome-derived cytokine IL18 suppresses amyloid-induced seizures in Alzheimer-prone mice.PMID:30127003
pharmacological inhibition of PARP-1 reversed both particulate matter-induced Abeta increase and glial activation.PMID:29654761
The concentrations of Abeta (1-42) were also significantly higher in early stage Alzheimer's disease (AD) mice compared with WT mice, however, the levels were markedly lower compared with later stage AD mice, as determined by ELISA. In addition to increased levels of Abeta (1-42) in mice with later stage AD, reduced astrocyte staining was observed compared with WT mice.PMID:29568933
work expands the current knowledge regarding Abeta seeding and the consequences thereof and attributes microglia an important role in diminishing Abeta seeding by environmental enrichment.PMID:29229786
This study demonstrated that APP as a novel receptor for Slit ligand mediating axon guidance and neural circuit formation.PMID:28785723
In vivo, the NHE6 knockout (NHE6(KO)) mouse model showed elevated Abeta in the brain, consistent with a causal effect. Increased nuclear translocation of histone deacetylase 4 (HDAC4) in ApoE4 astrocytes, compared with the nonpathogenic ApoE3 allele, suggested a mechanistic basis for transcriptional down-regulation of NHE6.PMID:29946028
This commentary reviews the role of the Alzheimer amyloid peptide Abeta on basal synaptic transmission, synaptic short-term plasticity, as well as short- and long-term potentiation in transgenic mice, with a special focus on N-terminal truncated Abeta4-42.PMID:29561816
ADAP KO mice developed glomerular pathology. ADAP KO podocytes lack cell protrusions with actin cytoskeleton forming circumferential stress fibers.PMID:29192064
Therefore, APP modulates Nav1.6 sodium channels through a Go-coupled JNK pathway, which is dependent on phosphorylation of APP at Thr668.PMID:28008944
These findings suggest that in the absence of CLU, Abeta clearance shifts to perivascular drainage pathways, resulting in fewer parenchymal plaques but more CAA because of loss of CLU chaperone activity, complicating the potential therapeutic targeting of CLU for AD.PMID:28701379
Chronic Dyrk1 inhibition reversed cognitive deficits in Alzheimer's disease transgenic mice via reduction of APP and phosphorylated tau pathology.PMID:28779511
The findings provide a model for initiation of synaptic dysfunction whereby exposure to physiologic levels of amyloid beta for a prolonged period of time causes microstructural changes at the synapse which result in increased transmitter release, failure of synaptic plasticity, and memory loss.PMID:27581852
The results of the present study substantiate that cGMP has a role in the endocytic pathway of APP and suggest a scenario where the cyclic nucleotide enhances the production of Abeta by favoring the trafficking of APP from the cell cortex to the endolysosomal compartment.PMID:28789837
Study showed that the APP Osaka mutation has dual effects: it causes a loss-of-function of APP and gain-of-toxic-function of Abeta, though the latter seems to come out only after the former causes GABAergic depletion. Also present OSK-KI mice as a mouse model to replicate the hereditary form of recessive familial Alzheimer's disease.PMID:28760161
Results show that the duration of UP state, which is a key feature of cortical synaptic integration occurring predominantly during slow-wave sleep, is significantly increased in the prefrontal cortex in the absence of APP. This was accompanied by a specific reduction in the glutamine synthetase and tissue GABA content and sequential upregulation in the levels of GABA-B receptor expression.PMID:27552836
results support the hypothesis that the miR-132/212 network, including Sirt1 and likely other target genes, contributes to abnormal Abeta metabolism and senile plaque deposition in AD.PMID:27484949
Activation of CaMKIV by soluble amyloid-beta1-42 impedes trafficking of axonal vesicles and impairs activity-dependent synaptogenesisPMID:28698220
Abpp /KPI(R13I) mutant mice were similarly deficient as Abpp knock out mice in regulating cerebral thrombosis in experimental models of carotid artery thrombosis and intracerebral hemorrhage.PMID:28499154
The cognitive function of APP/PS1 mice was impaired at 10months of age; moreover, the hypermetabolic state identified in various brain regions at 5months of age was also significantly decreased.PMID:29107091
APP heterozygosity results in greater decreases of cortical APP in Transgenic (Tg) versus non-Tg mice. Mutant huntingtin transgenic mice develop brain iron accumulation as a result of greater suppression of APP levels. Elevated brain iron in Tg mice was associated with a decline in motor endurance consistent with a disease promoting effect of iron in the YAC128 model of human Huntington's Disease.PMID:28550267
Mass spectrometry analysis of APP intracellular domains revealed differential processing of APP-C83, APP-C89, and APP-C99 by gamma-secretase already at the epsilon-cleavage stage. This mechanistic insight could aid in developing substrate-targeted modulators of APP-C99 processing to specifically lower the Abeta42:Abeta40 ratio without compromising gamma-secretase function.PMID:28591569
Data show that exosomal amyloid precursor protein C-terminal fragments (APP-CTFs) and bis(monoacylglycero)phosphate (BMP) as candidate biomarkers diagnostic of endolysosomal dysfunction associated with neurodegenerative disorders.PMID:29348617
study provides molecular insights into the design of amyloidogenic inhibitors to cure various neurodegenerative and amyloid-associated diseases, as NABi would regulate aggregation of other toxic beta-sheet proteins other than Abeta.PMID:29107146
Conducted in vivo extracellular recording to investigate cholinergic compound action potentials of the superior cervical ganglion (SCG) in APP(-/-) and littermate wild-type (WT) mice; found that APP not only regulates presynaptic activity, but also affects postsynaptic function at cholinergic synapses in SCG; also alpha4beta2 and alpha7 nicotinic acetylcholine receptors are reduced in the absence of APP.PMID:27553120
App-KI mouse lines with different levels of pathophysiology are useful models of AD.PMID:27377630
Loss of Abpp is associated with cognitive impairment.PMID:27049828
long term survival and amyloid protein levels are modified by positive and negative early life experiences in a mouse model of Alzheimer's diseasePMID:27259247
the synaptic localization of APP, ADAM10, and BACE1 in the mouse cerebral cortex, was examined.PMID:26497029
Taken together, these results suggest that apoE-containing discoidal HDLs do not require LCAT-dependent maturation to mediate efficient Abeta clearancePMID:24950691
APP knockout mice have shorter dendritic arbors in the hippocampus.PMID:27664851
This study demonstrates the neuroprotective effect of TSG on APP expression, suggesting that TSG may be beneficial for AD prevention and treatment.PMID:29129695
SNX15 regulates the recycling of APP to cell surface and, thus, its processing for Abeta generation.PMID:26115702
Immunohistochemical analysis confirmed increased amount of NOS1 protein in neuronal somata and processes in the perilesional cortex in APP/PS1-severe traumatic brain injury(TBI) mice compared to APP/PS1-sham (p < 0.05) or Wt-sTBI mice (p < 0.01).PMID:26671618
Combining a murine APP-deficient and a human APP-transgenic strain, we were able to analyse the progression of the cortical amyloidosis independent of the murine variant. The lack of endogenous mAPP resulted in accelerated deposition and, thus, increased number of senile plaques and higher levels of aggregated hAbeta.PMID:28637503
our findings indicate that sortilin is a beneficial protein for the reduction of amyloid pathology in APP/PS1 mice by promoting APP degradationPMID:29056359
APP levels then decrease progressively as a function of age in close relationship with the gradual normalization of FMRP and hnRNP C levels.PMID:26048669
a 99-aa C-terminal fragment of APP,C99, in addition to its localization in endosomes, can also be found in mitochondria-associated endoplasmic reticulum (ER) membranes, where it is normally processed rapidly by gamma-secretase.PMID:29018038
The authors concluded that the FcgammaRIIb-SHIP2 axis links Abeta neurotoxicity to tau pathology by dysregulating phosphoinositide metabolism, providing insight into therapeutic potential against Alzheimer's disease.PMID:27834631
results suggest that PrP(C) recognizes structural features common to both Abeta oligomers and fibril ends and that this interaction could contribute to the neurotoxic effect of Abeta aggregates.PMID:28842494
Our study provides the first direct evidence that Abeta, an AD-linked factor, is associated to the pathogenesis of ALS and provides molecular clues to understand common aggregation mechanisms in the pathogenesis of neurodegenerative diseases.PMID:28864422
These data provide evidence that amyloid beta acts to enhance tau pathology by increasing the formation of tau species capable of seeding new aggregates.PMID:28500862
Although hyperactivity and hypersynchronicity were respectively detected in mice expressing the PS2-N141I or the APP Swedish mutant alone, the increase in cross-frequency coupling specifically characterized the 6-month-old PS2APP mice, just before the surge of the cognitive declinePMID:27889678
these results uncover a novel role for mDia1 in Abeta-mediated synaptotoxicity and demonstrate that inhibition of MT dynamics and accumulation of PTMs are driving factors for the induction of tau-mediated neuronal damage.PMID:28877993
APP and its metabolites are capable of influencing the basic physiology of the pancreas.PMID:28710249
Show
More
Hide
All
Subcellular Location
Cell membrane; Single-pass type I membrane protein. Membrane; Single-pass type I membrane protein. Perikaryon. Cell projection, growth cone. Membrane, clathrin-coated pit. Early endosome. Cytoplasmic vesicle. Golgi apparatus, trans-Golgi network.; [C99]: Early endosome.; [C83]: Endoplasmic reticulum. Golgi apparatus. Early endosome.; [Soluble APP-beta]: Secreted.; [Amyloid-beta protein 42]: Cell surface.; [Gamma-secretase C-terminal fragment 59]: Nucleus. Cytoplasm.
Protein Families
APP family
Tissue Specificity
Expressed in the brain with expression in cortex, cerebellum, hippocampus, olfactory bulb, neurons, astrocytes and microglia (at protein level). Expressed in the retinal lens. Expressed at a low level in muscle cells (at protein level).; [Isoform APP770]: